

 Inglês (pdf)
 Artigo em XML
 Referências do artigo

 Tradução automática
 Enviar este artigo por email
 Citado por SciELO
 Similares em
SciELO

 Permalink

INTRODUCTION
Cyanobacteria are photoautotrophic organisms naturally found in aquatic ecosystems, including rivers, streams, reservoirs, and lakes, where they constitute the phytoplankton community alongside microalgae and maintain the foundation of aquatic trophic dynamics1. Beyond their ecological role, phytoplankton assemblages serve as sensitive bioindicators, enabling the identification of specific environmental changes through analyses of species composition and distribution patterns2,3.
Under conditions of increased nutrient availability, caused by natural processes or human activities, cyanobacteria proliferate rapidly, leading to blooms that significantly alter water quality. These blooms affect the organoleptic properties of water and pose serious risks to human health by producing and releasing cyanotoxins4. The presence of toxic cyanobacteria in water bodies has been associated with various health issues, including cases of liver failure in children5, raising concerns for both drinking water sources and recreational activities, as exposure may occur through direct contact during bathing or other aquatic activities. Climate change scenarios may intensify these occurrences by extending periods of thermal stratification, increasing nutrient concentrations due to altered water flow, and creating favorable conditions for harmful blooms6.
Cyanobacterial proliferation compromises the recreational use of water bodies, such as rivers and beaches, underscoring the need for continuous monitoring and management actions to mitigate environmental and public health impacts7. This challenge is particularly critical for riverside cities, where the effects of climate change may demand rapid responses to protect human populations and aquatic ecosystems.
Recent studies at Lago Grande do Curuai, in Santarém Municipality, Pará State, Brazil, have identified critical ecological thresholds associated with turbidity, temperature, pH, total nitrogen, and precipitation, showing that species respond directly to these gradients and are favored by high temperatures, nutrients, and turbidity8. In Pará, taxonomic surveys have recorded 153 cyanobacteria taxa in freshwater and coastal environments, mainly from the families Merismopediaceae, Oscillatoriaceae, and Microcystaceae9. Across the Brazilian Amazon, 145 freshwater species have been reported, with Microcystis and Planktothrix being the most frequent genera, often associated with toxic blooms and microcystin production, even at low cell densities10,11. However, systematic data from the Amazon remain scarce, limited by logistical and infrastructural challenges that hinder continuous research.
The Pará River, in Pará State, which borders the Caripi, Itupanema, and Conde beaches, typically does not favor cyanobacterial blooms due to its dynamic hydrology, tidal currents, high flow volume, and slightly acidic to alkaline and turbid waters. However, recorded bloom events in 202212 suggest that anthropogenic pressures may override these natural barriers.
Predicted changes in the Amazonian hydrological regime due to climate change, such as intensified droughts and floods, may further reduce phytoplankton dispersal and dilution capacity, thereby increasing the likelihood of blooms even in environments previously considered unfavorable. However, little is known about the factors that promote blooms in Amazonian waters, as this is a rare event, with more records in the Pará and Tapajós rivers, in Santarém11,13.
Since 2000, the Pará River region, situated between the municipalities of Barcarena and Abaetetuba, has experienced a series of environmental accidents, including oil spills, red mud discharges, coke releases, and shipwrecks, resulting in severe water pollution. Such conditions increase the vulnerability of local ecosystems to cyanobacterial blooms, which have already been recorded on local beaches12.
It is essential to understand the dynamics of phytoplanktonic cyanobacteria along Barcarena's beaches, as well as the factors associated with bloom formation, to support water quality monitoring and management. Continuous monitoring of bacterial density at beaches such as Conde, Caripi, and Itupanema is necessary, given the scarcity of studies on the Pará River. In addition, the interaction between climatic variables and anthropogenic pressures must be considered to anticipate risks and guide mitigation and adaptation measures in response to climate change.
Thus, the study aimed to determine the spatiotemporal variation of cyanobacteria on the beaches of Barcarena, Pará State, in relation to physicochemical, water-nutrient, and climatological variables, identifying variables responsible for cyanobacterial dynamics and assessing the water quality of the beaches in accordance with CONAMA Resolution No. 274/2000.
MATERIALS AND METHODS
STUDY AREA AND SAMPLE DESIGN
The Pará River estuary, one of the largest in Brazil, extends over 320 km and has a mouth approximately 60 km wide. The Tocantins, Guamá, and Acará-Moju rivers are its main tributaries, contributing significantly to water and sediment flow and shaping estuarine dynamics. The region is subject to significant tidal variations, with amplitudes ranging from 5 m at the mouth to 1.5 m in its interior, and an average fluvial discharge of 10⁴ m³/s approximately7,14-17.
The estuary is influenced by the Atlantic Ocean tides and the region's climate, classified as hot and humid (Am) according to the Köppen classification, with an average annual temperature of 26 ºC, relative air humidity consistently above 80%, and well-defined seasonality. The rainy season (December-May) corresponds to higher river flow, while the dry season (June-November) results in lower discharge and increased salinity in the Pará River estuary, providing oligohaline waters17-20.
The beaches of Vila do Conde, Itupanema, and Caripi attract numerous residents and tourists for leisure, recreation, and relaxation. However, water quality in these coastal environments can be significantly affected by various anthropogenic factors21. Unregulated urban expansion, intense port activities involving the arrival of vessels from around the world, and the presence of large mining industries in the Barcarena area further exacerbate this issue. Incidents of mine tailings spills have been reported, releasing toxic metals into the Pará River22,23.
COLLECTION AND ANALYSIS OF CYANOBACTERIA
Samples were collected from three beaches in Barcarena: Caripi (01°29'52.5"S 048°42'42.1"W), Itupanema (01°31'06.3"S, 48°43'45.8"W), and Conde (01°33'96.4"S, 048°46'13.6"W), in September 2021 and March 2022. Three equidistant collection points were selected at each beach (Figure 1). Samples of cyanobacteria, physicochemical variables, and chlorophyll-a were collected at the collector's breast height, following the procedures of CONAMA Resolution No. 274/200024.
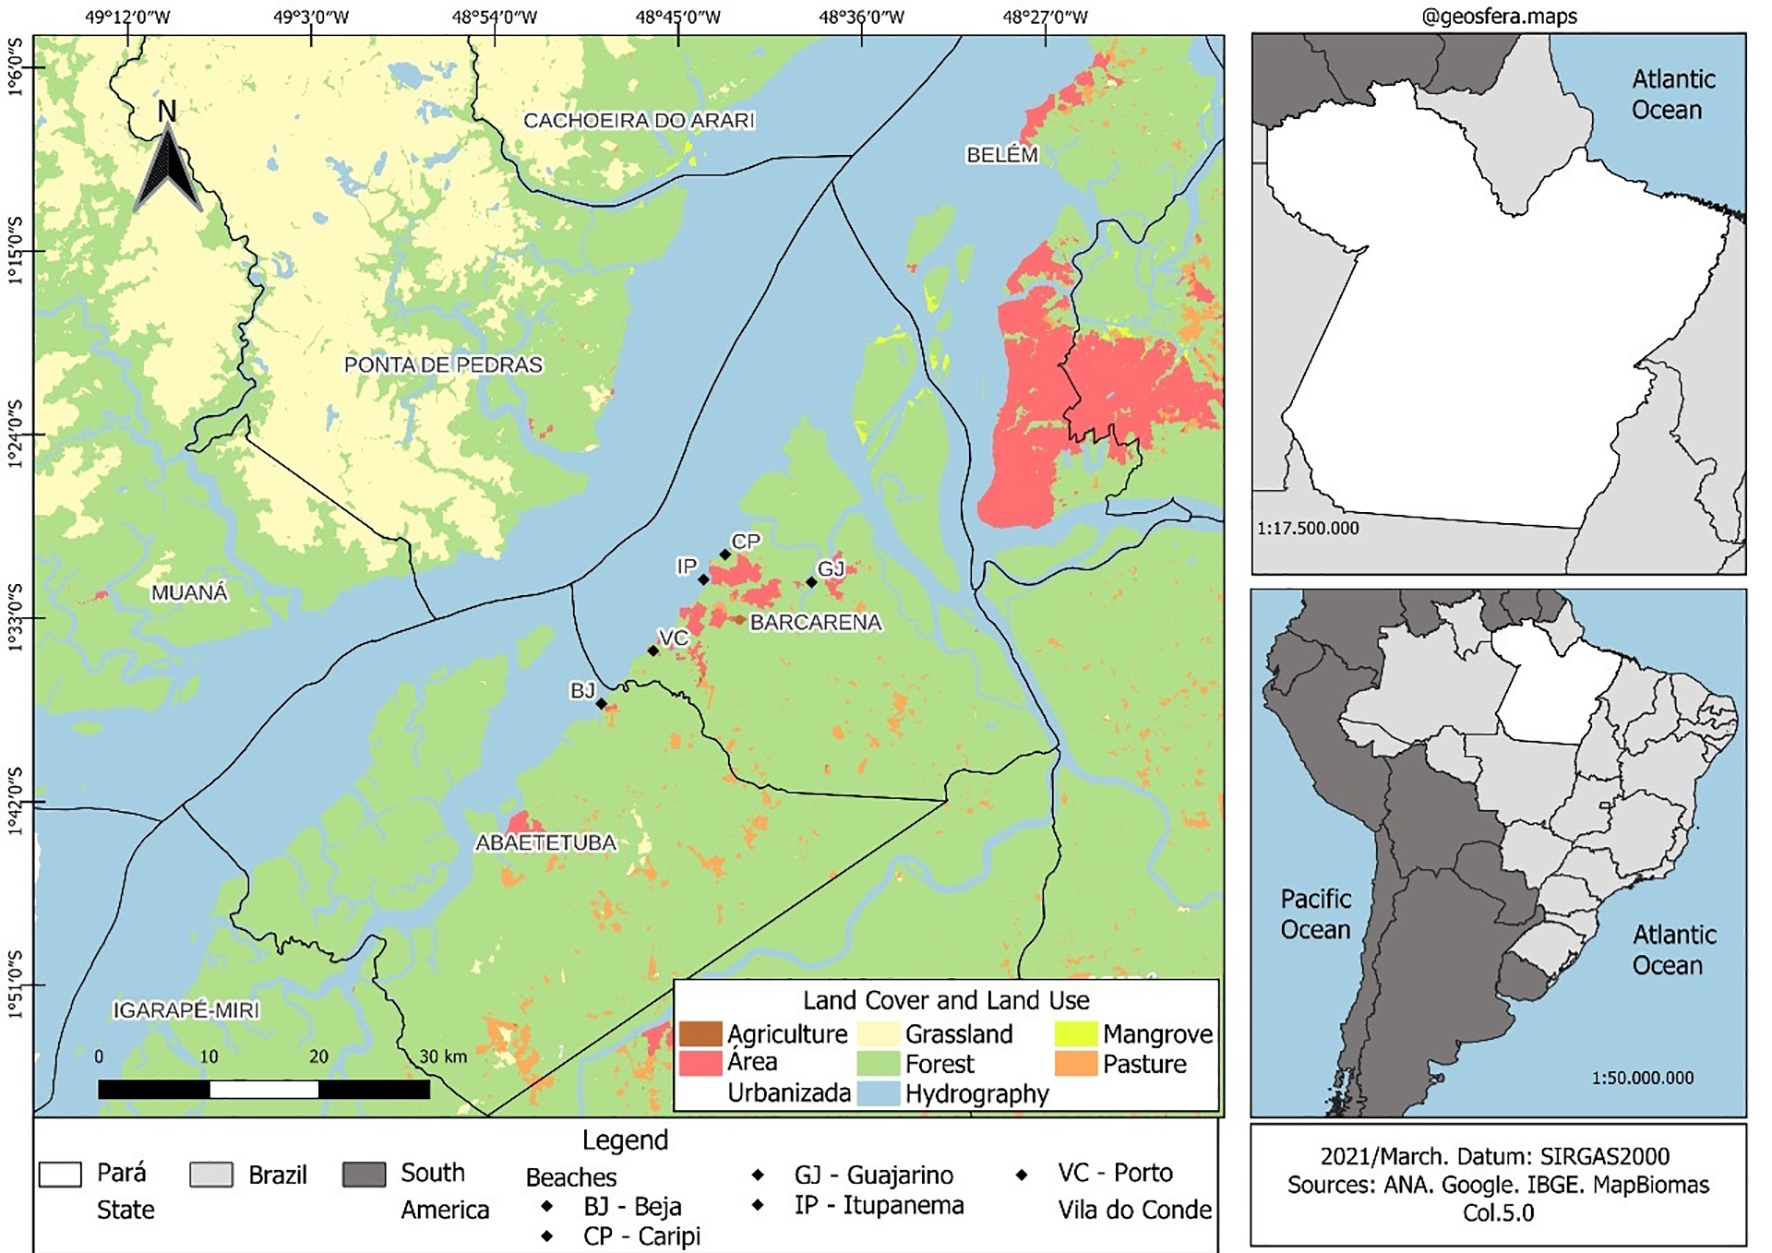
Source: Autor, 2025.
Figure 1 - Map of the study area in the Pará River estuary, showing the sampling sites (black diamonds) at Conde (VC), Itupanema (IP), and Caripi (CP) beaches, Barcarena, Pará State, Brazil
Cyanobacteria samples were collected from the water subsurface using 300 mL polypropylene bottles and fixed with formaldehyde. The Ütermohl sedimentation method21 was employed for the identification and counting of taxa, with the density expressed in cells·mL⁻¹ according to the 10200 F counting technique25. Analyses were performed on an Axiovert 40C inverted microscope coupled to an image capture system (AxioCam MRc, Carl Zeiss). Identification, nomenclature, and taxonomic framework were performed according to the specialized literature26,27,28.
The frequency of occurrence was calculated according to Matteucci and Colma29. Relative abundance (A) of each taxon was determined using the formula A = (N × 100) / N_total, where "N" is the number of individuals of a given taxon and "N_total" is the total number of individuals in the sample. Taxa representing more than 50% of the total individuals were classified as dominant, while those with values above the mean abundance were considered abundant30.
COLLECTION AND ANALYSIS OF CHLOROPHYLL-A, B, AND C
Chlorophyll samples were collected from the water subsurface in 1.000 mL amber polypropylene bottles and stored in isothermal boxes at 4 ºC. Subsequently, chlorophyll extraction was followed by filtration through cellulose filters with a 0.45 µm pore size, with the retained material macerated in 90% acetone as described in Standard Methods for the Examination of Water and Wastewater (APHA)25. The samples were analyzed by spectrophotometry (DR 6000, HACH), following method 10200 F.
COLLECTION AND ANALYSIS OF NUTRIENTS AND PHYSICOCHEMICAL VARIABLES
Water temperature (°C), hydrogen potential (pH), salinity (PSU), electrical conductivity (EC), total dissolved solids (TDS), and dissolved oxygen (DO) were measured using a multiparameter probe (HI 9828, HANNA®, USA). For the other variables, water samples were collected in glass bottles following APHA recommendation 106025. Turbidity, apparent color, and true color were determined using the nephelometric method 2130 B25, while total suspended solids (TSS) were quantified photometrically.
Chemical oxygen demand (COD) was analyzed by method 5220 D of the APHA25 using UV-VIS spectrometry (model DR 3900). Nutrients nitrate (NO₃⁻), chloride (Cl⁻), and sulfate (SO₄²⁻) were determined by ion chromatography (ICS Dual 2000, Dionex Corporation, Sunnyvale, CA, USA) following method 4110 B25. Alkalinity was calculated by the titrimetric method 2320 B25.
CLIMATOLOGICAL VARIABLES
Precipitation and wind speed data were obtained from the Belém meteorological station (1°25'48.0"S, 48°25'12.0"W) and provided by the National Institute of Meteorology (INMET).
LEGISLATION
The analyzed legislation included CONAMA Resolution No. 357/200531, which regulates the classification and framework of water bodies, and CONAMA Resolution No. 274/2000, which establishes the criteria for bathing water quality in Brazil. For Class 2 freshwaters, applicable to the Pará River due to its multiple uses, CONAMA Resolution No. 357/2005 sets the following limits: pH (6.0-9.0), DO (≥ 5 mg·L⁻¹), TDS (≤ 500 mg·L⁻¹), turbidity (≤ 100 NTU), true color (≤ 75 mg Pt·L⁻¹), chloride (≤ 250 mg·L⁻¹), sulfate (≤ 250 mg·L⁻¹), nitrate (≤ 10 mg·L⁻¹ as N-NO₃⁻), COD (≤ 90 mg·L⁻¹ O₂), chlorophyll-a (≤ 30 µg·L⁻¹), and cyanobacteria density (≤ 50,000 cells·mL⁻¹). These parameters guided the assessment of water quality and the occurrence of cyanobacterial blooms. CONAMA Resolution No. 274/2000, applied to the beaches of Barcarena, establishes bathing water classifications, considering waters unsuitable when visible blooms of microalgae, particularly cyanobacteria, are present, especially when associated with color changes or scum formation that compromises recreational use.
DATA ANALYSIS
Multivariate analyses included principal component analysis (PCA) and redundancy analysis (RDA). PCA, based on Euclidean distance, was used to assess the sample distribution and correlations among physicochemical, biomass (chlorophyll), and climatological variables, all standardized to normalized values (ranging values) to minimize scale effects. RDA was performed using an abiotic matrix and a biological matrix composed of the most abundant species, excluding those with relative abundance ≥ 5%32. The biological matrix was Hellinger-transformed33 to reduce the influence of dominant species and account for zero inflation. Multivariate analyses were performed in CANOCO 4.5 for Windows34.
RESULTS
BIOLOGICAL VARIABLES
Composition
A total of 41 cyanobacterial species were identified, distributed across four orders and 14 families. In September 2021, 23 species from six families were found. The most representative families were Merismopediaceae (26%), Microcoleaceae (26%), and Aphanizomenonaceae (13%). The most frequent species, being present on all beaches, were: Anagnostidinema amphibium (Agardh ex Gomont, 1892) Strunecký et al., 2017; Aphanizomenon gracile Lemmermann, 1907; Cuspidothrix sp.; Cyanogranis ferruginea (F.Wawrik) Hindák ex Hindák 2006; Merismopedia tenuissima Lemmermann, 1898 in [Lemmermann E (1898b)]; Planktolyngbya limnetica (Lemmermann, 1898) Komárková-Legnerová & Cronberg, 1992 in [Komárková-Legnerová J. & Cronberg, G. (1992)]; and Pseudanabaena limnetica (Lemmermann 1900) Komárek 1974.
In March 2022, 33 cyanobacterial species belonging to 12 families were found. The most representative families were Merismopediaceae (26%), Oscillatoriaceae (17%), and Aphanizomenonaceae (11%). The most frequent species were Anagnostidinema amphibium, Aphanizomenon sp., Aphanocapsa delicatissima W.West & G.S.West, Merismopedia tenuissima, Phormidium lividum (Hansgirg) Forti, and Planktolyngbya limnetica, which occurred on all beaches. Caripi Beach showed the highest species richness (14 taxa), while Conde Beach had the lowest (eight taxa).
Density
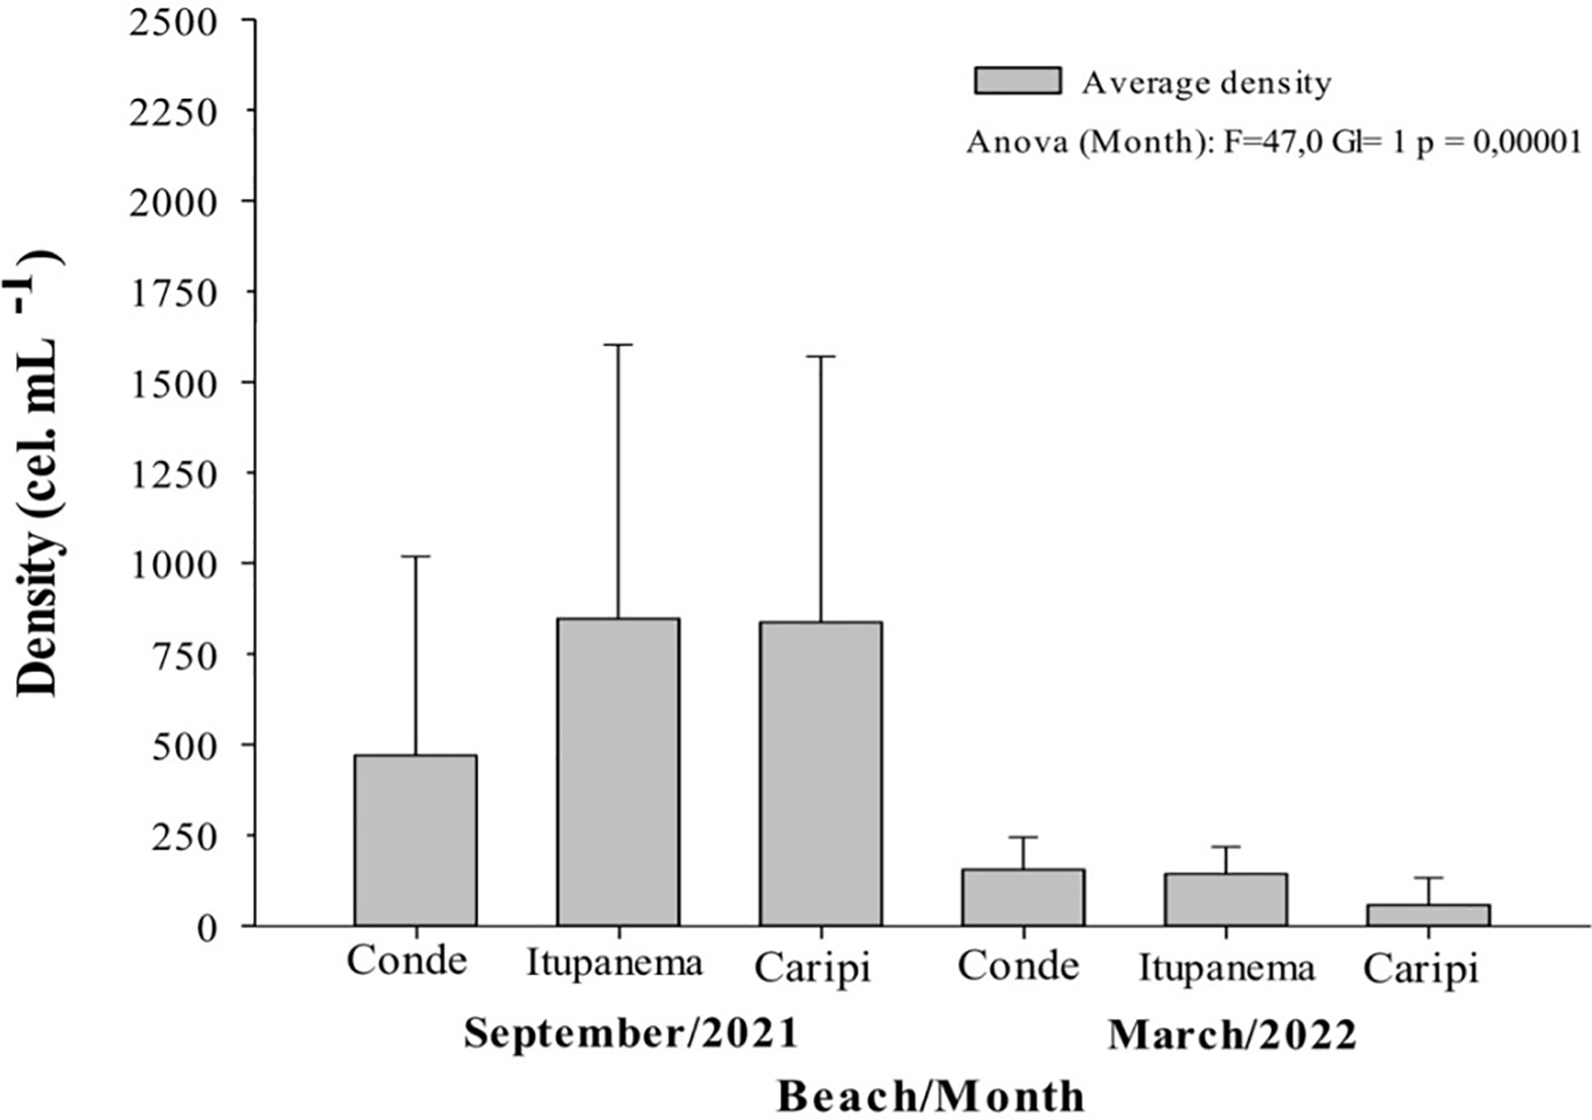
Temporal and spatial patterns in cyanobacterial density and composition were observed across sampled beaches (Figure 2). Overall, cyanobacterial density was higher in September 2021 (1,495.0 ± 298.0 cells·mL⁻¹) than in March 2022 (220.3 ± 79.3 cells·mL⁻¹). In September 2021, Conde Beach presented the lowest density (490.0 ± 304.0 cells·mL⁻¹), whereas in March 2022, the lowest values were recorded at Caripi Beach (140.3 ± 7.4 cells·mL⁻¹).
Source: Autor, 2025.
Figure 2 - Spatiotemporal variation in the mean density of cyanobacteria at Amazonian fluvial-estuarine beaches in Barcarena, Pará State, Brazil
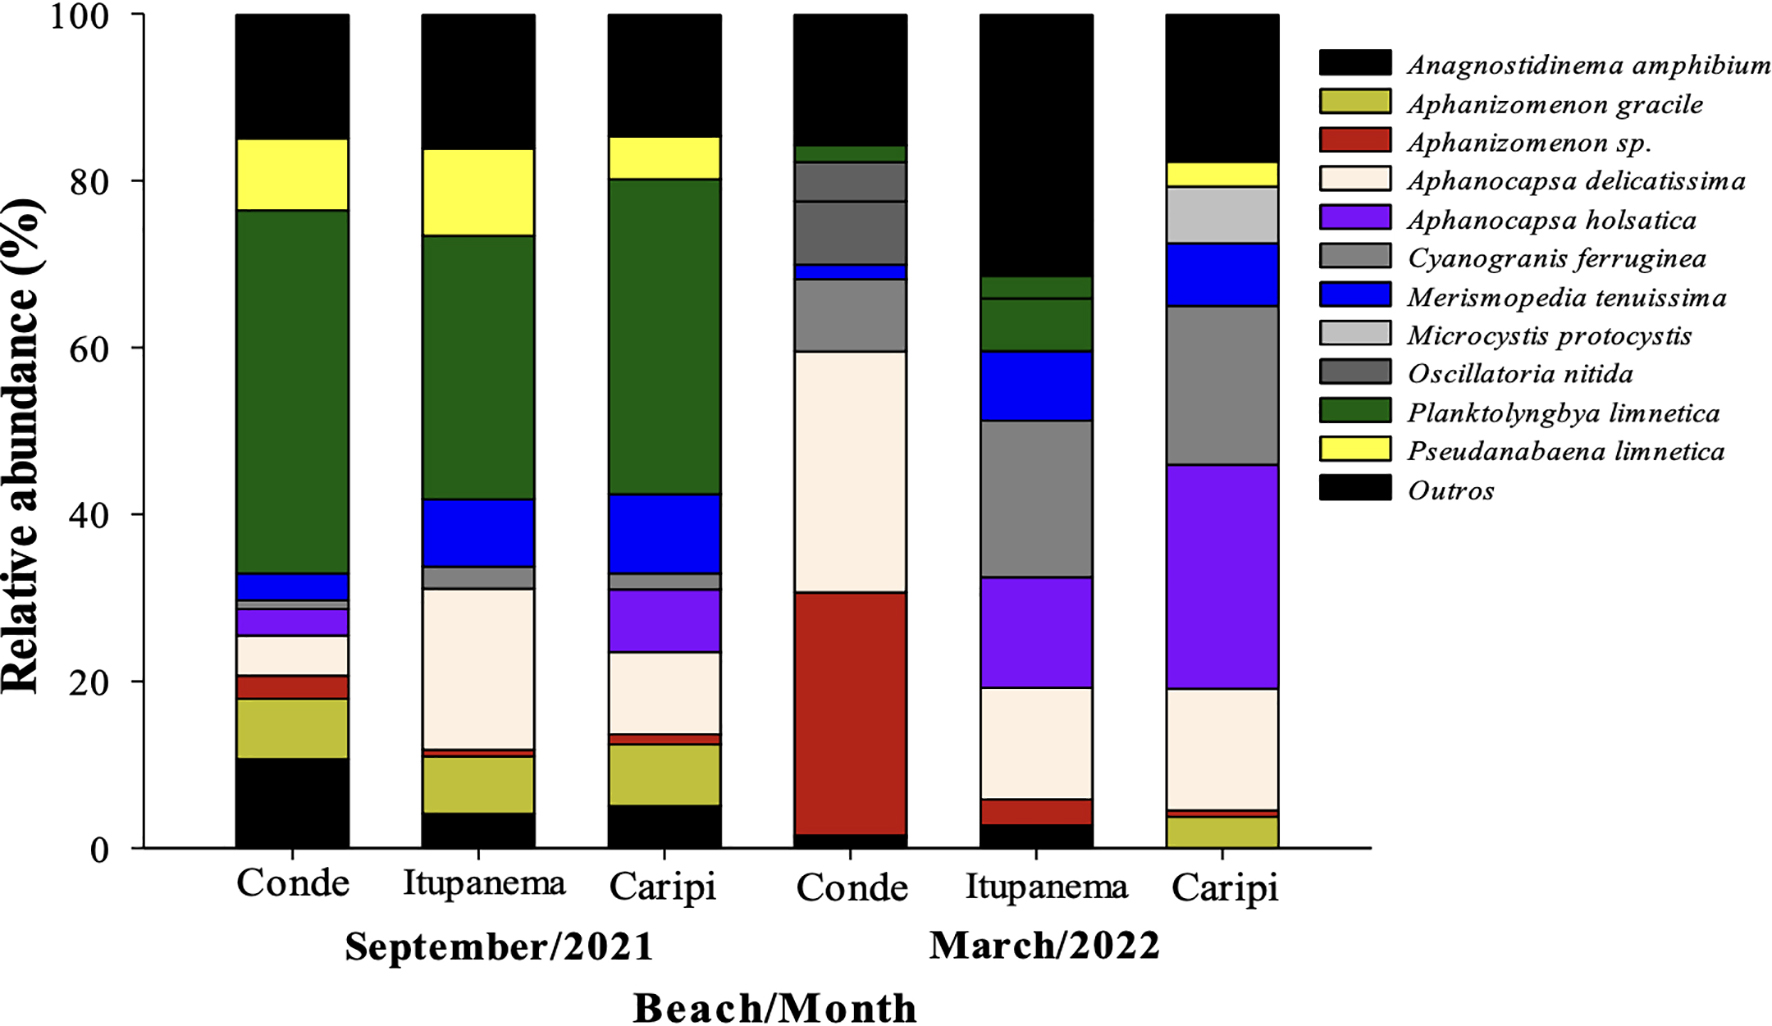
Regarding relative abundance, 11 species stood out as abundant throughout the period and sites (Figure 3). In September 2021, Planktolyngbya limnetica was the most abundant species, whereas in March 2022, Aphanocapsa delicatissima, Aphanizomenon gracile, and Aphanocapsa holsatica (Lemmermann) G. Cronberg & Komárek 1994 predominated.
ENVIRONMENTAL VARIABLES
Descriptive analyses of the limnological factors are listed in Table 1. Physicochemical parameters showed both temporal and spatial variation across sampling periods and beaches.
Table 1 - Temporal variation in the physicochemical variables of Amazonian fluvial-estuarine beaches in Barcarena, Pará State, Brazil
| Physicochemical parameters | September 2021 | March 2022 | CONAMA Resolution No. 357/2005 |
|---|---|---|---|
| Min.-max. (mean ± SD); median | Min.-max. (mean ± SD); median | ||
| pH | 6.8-7.2 (7.1 ± 0.1); 7.1 | 6.6-6.9 (6.8 ± 0.1); 6.8 | 6.0 a 9.0 |
| T (°C) | 28.9-30.6 (29.7 ± 0.6); 29.9 | 28.9-30.1 (27.4±6.9); 29.8 | N/A |
| EC (µS·cm⁻¹) | 44.0-62.0 (52.3 ± 7.3); 52.0 | 41.0-74.0 (55.8 ± 12.1); 58.0 | N/A |
| TDS (mg·L⁻¹) | 22.0-31.0 (26.2 ± 3.8); 26.0 | 29.0-52.0 (39.2 ± 8.6); 41.0 | ≤ 500.0 mg·L⁻¹ |
| Sal (PSU) | 0.0-0.02 (0.0 ± 0.0); 0.0 | 0.0-0.01 (0.0 ± 0.0); 0.0 | N/A |
| DO (mg·L⁻¹) | 5.4-6.9 (6.1 ± 0.5); 6.1 | 3.1-4.4 (3.6 ± 0.4); 3.6 | ≥ 5 mg·L⁻¹ |
| TSS (mg·L⁻¹) | 6.0-13.0 (9.1 ± 2.2); 9.0 | 8.0-17.0 (12.2 ± 3.0); 12.0 | N/A |
| Turb (UNT) | 8.0-16.0 (12.3 ± 2.9); 12.5 | 12.1-29.5 (19.2 ± 4.7); 18.3 | 100 UNT |
| AC (mg·L⁻¹) | 85.0-135.0 (105.6 ± 16.7); 107.5 | 95.0-160.0 (124.8 ± 17.5); 123.0 | N/A |
| TC (mg·L⁻¹) | 21.0-29.0 (26.0 ± 3.2); 27.0 | 33.0-45.0 (37.7 ± 4.3); 38.0 | ≤ 75.0 mg Pt-Co·L⁻¹ |
| Alka (mg·L⁻¹) | 8.0-15.0 (10.6 ± 2.1); 10.0 | 40.0-80.0 (56.7 ± 14.1); 50.0 | N/A |
| COD (mg·L⁻¹) | 19.0-41.0 (30.9 ± 6.5); 31.0 | 0.0-18.0 (5.3 ± 7.1); 0.0 | N/A |
| Cl⁻ (mg·L⁻¹) | 0.7-1.6 (1.1 ± 0.3); 1.0 | 3.0-7.4 (4.7 ± 1.5); 4.9 | ≤ 250.0 mg·L⁻¹ |
| NO₃⁻ (mg·L⁻¹) | 0.0-0.1 (0.1 ± 0.0); 0.1 | 0.0-0.2 (0.1 ± 0.1); 0.1 | ≤ 10.0 mg·L⁻¹ |
| SO₄²⁻ (mg·L⁻¹) | 0.4-4.6 (1.7 ± 1.3); 1.5 | 0.0-4.5 (2.5 ± 1.7); 2.2 | ≤ 250.0 mg·L⁻¹ |
| Chl-a (µg·L⁻¹) | 4.5-14.2 (8.5 ± 3.4); 7.5 | 2.0-5.3 (3.8 ± 1.7); 4.0 | 30 μg·L⁻¹ |
| Chl-b (µg·L⁻¹) | 0.4-1.3(0.7 ± 0.3); 0.6 | 1.1-2.1 (1.5 ± 0.6); 1.2 | N/A |
| Chl-c (µg·L⁻¹) | 1.0-2.1 (1.5 ± 0.4); 1.7 | 1.4-1.7 (1.5 ± 0.2); 1.6 | N/A |
pH: Hydrogen potential; T: Temperature; Sal: Salinity; Turb: Turbidity; AC: Apparent color; TC: True color; Alka: Alkalinity; EC: Electrical conductivity; TDS: Total dissolved solids; DO: Dissolved oxygen; TSS: Total suspended solids; COD: Chemical oxygen demand; Cl⁻: Chloride; NO₃⁻: Nitrate; SO₄²⁻: Sulfate; Chl-a: Chlorophyll-a; Chl-b: Chlorophyll-b; Chl-c: Chlorophyll-c; N/A: Not applicable.
March waters showed higher concentrations of TDS, turbidity, apparent color, true color, alkalinity, chloride, nitrate, and TSS, and were slightly acidic and less oxygenated compared to September waters, which presented a more alkaline pH and higher COD.
Among the beaches, Conde Beach had the highest concentrations of TDS (47.7 ± 4.5 mg·L⁻¹), EC (67.7 ± 6.5 µS·cm⁻¹), apparent color (139.3 ± 18.9 mg·L⁻¹), and sulfate (4.0 ± 0.7 mg·L⁻¹). Only DO values were unsatisfactory during March 2022.
Rainfall was 36% lower in September 2021 (339.6 mm) than in March 2022 (527.4 mm), the region's wettest month. Wind speeds were lower in March 2022 (2.4 km·h⁻¹) than in September 2021 (4.2 km·h⁻¹).
Chlorophyll-a concentrations were higher in September 2021 (8.5 ± 3.4 µg·L⁻¹) compared to March 2022 (3.8 ± 1.7 µg·L⁻¹). Similarly, chlorophyll-c was higher in September 2021 (1.5 ± 0.4 µg·L⁻¹). Chlorophyll-b peaked in March 2022 (1.5 ± 0.6 µg·L⁻¹) and was lowest in September 2021 (0.7 ± 0.3 µg·L⁻¹) (Table 1).
PCA confirmed the spatiotemporal variation observed in the study area. The two main axes of the PCA explained 70% of the variations. PC1 (55.0%) represented the temporal gradient, separating the sampling periods. The positive quadrant grouped the March 2022 samples, which were correlated with chloride (0.29), TDS (0.27), alkalinity (0.28), and precipitation (0.29). In the negative quadrant, DO (-0.28) and wind speed (-0.29) were correlated with the September 2021 samples (dry period).
On the other hand, PC2 (15.0%) established a spatial pattern. The positive quadrant grouped the samples from Caripi Beach and the March samples from Itupanema Beach, which were correlated with EC (-0.49), salinity (-0.44), and sulfate (-0.45). Conversely, the Conde Beach samples correlated with the September samples from Itupanema Beach for the same environmental variables (Figure 4).
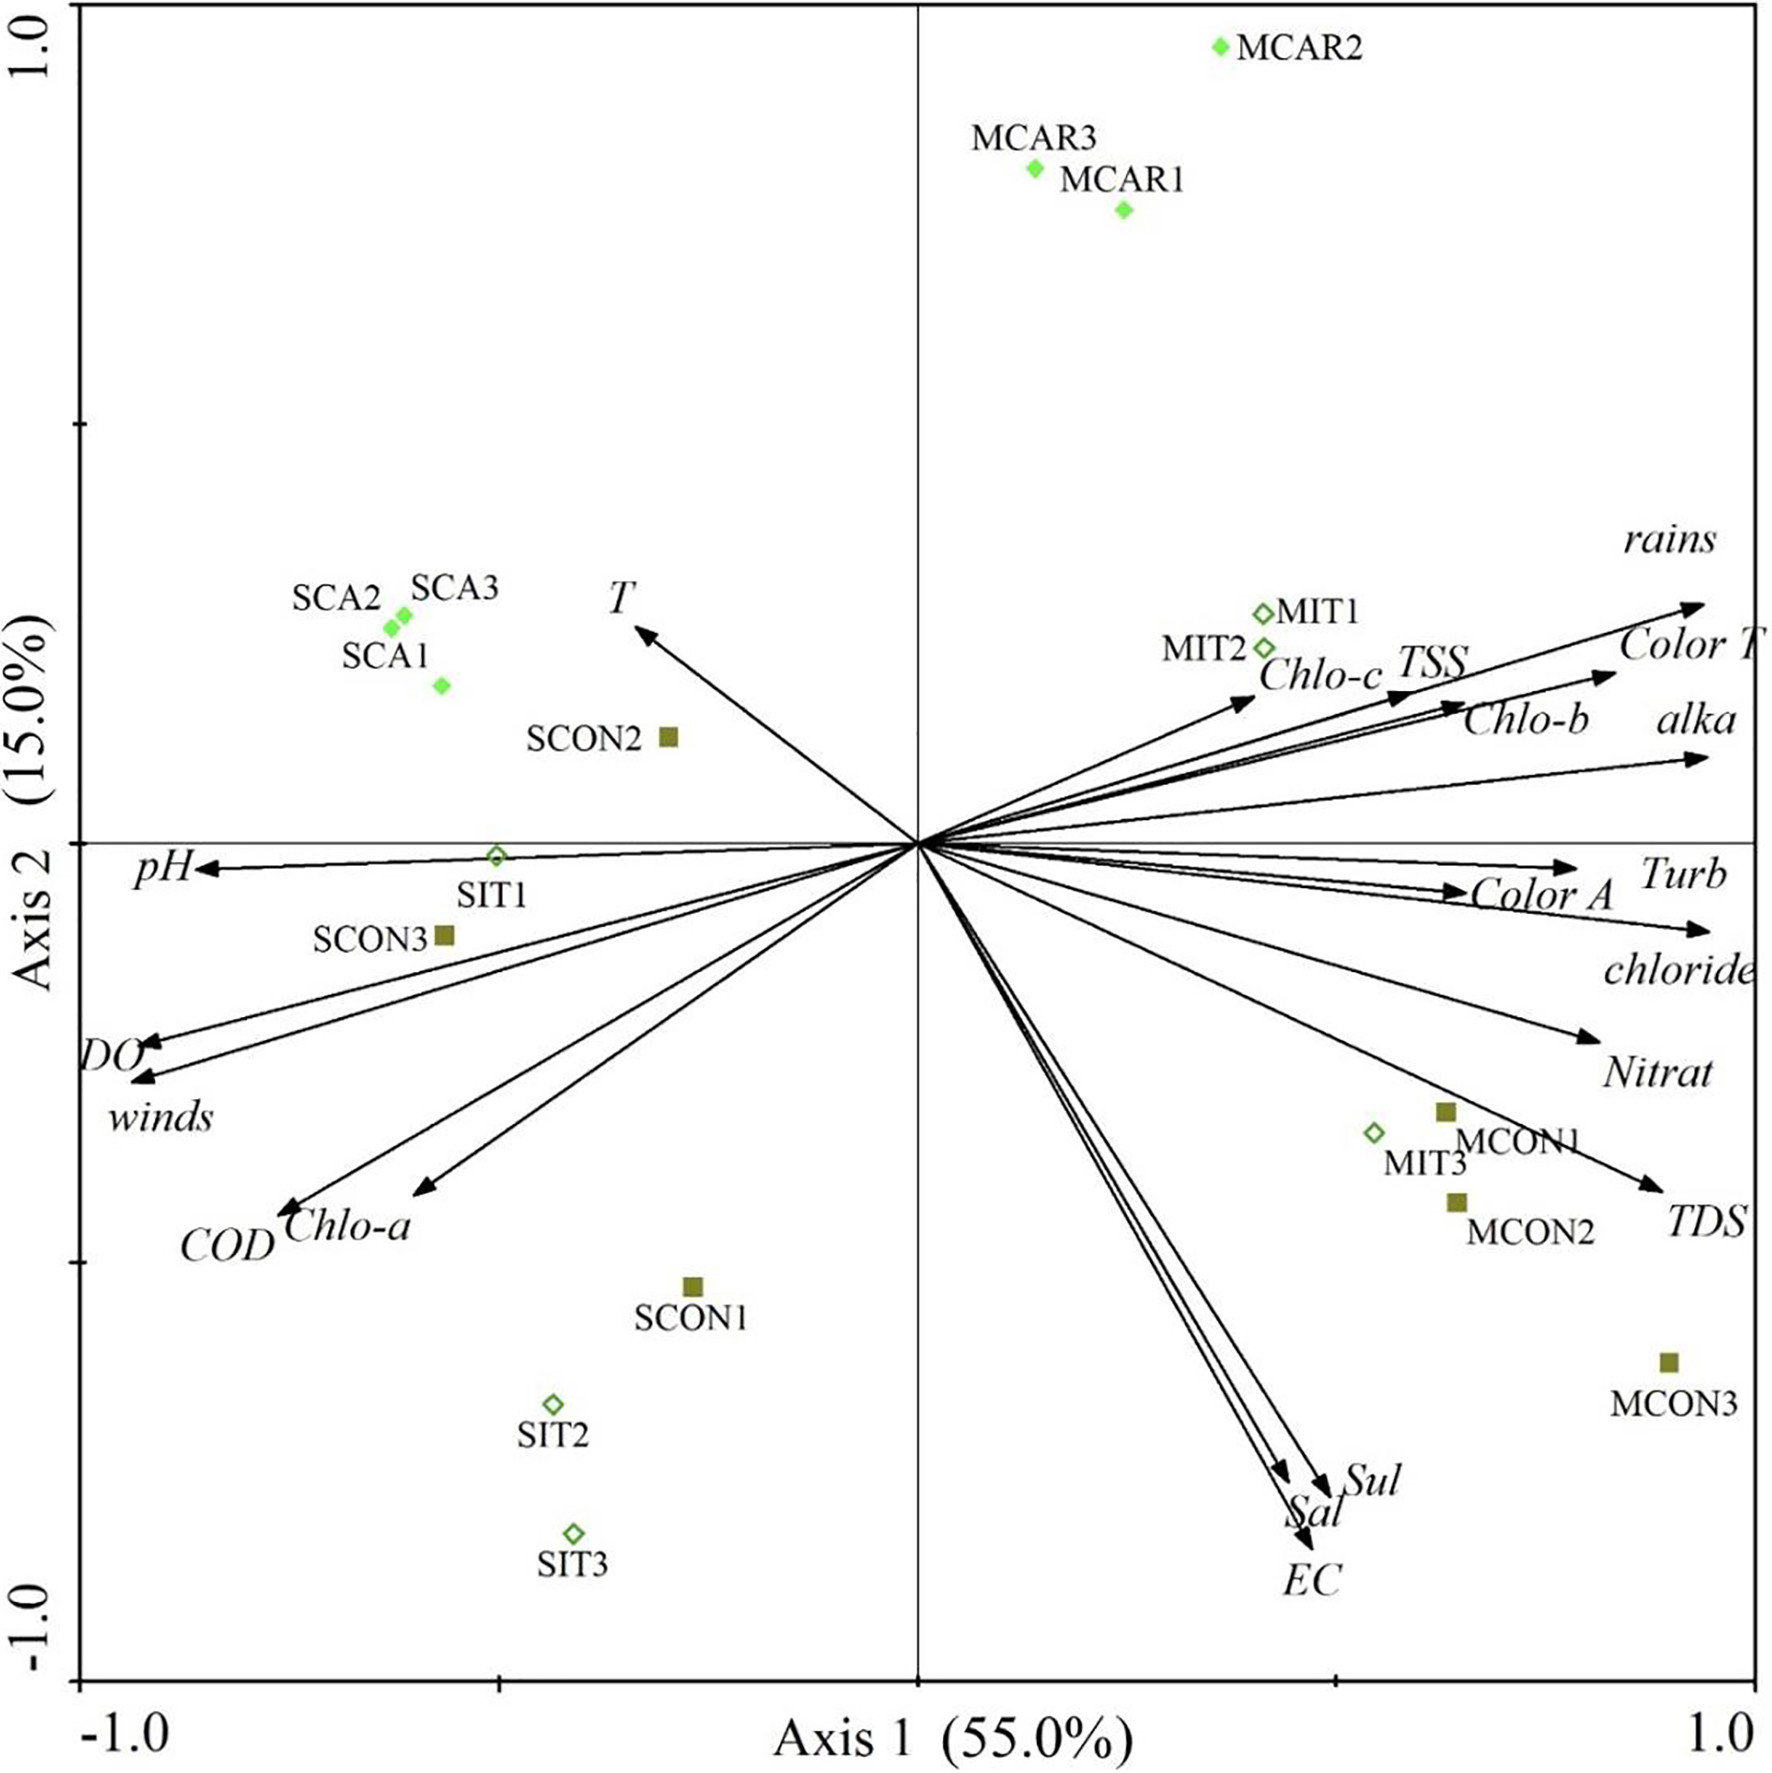
SCON: Conde Beach in September; SIT: Itupanema Beach in September; SCA: Caripi Beach in September; MCON: Conde Beach in March; MIT: Itupanema Beach in March; MCAR: Caripi Beach in March; pH: Hydrogen potential; EC: Electrical conductivity; TDS: Total dissolved solids; TSS: Total suspended solids; COD: Chemical oxygen demand; T: Temperature; DO: Dissolved oxygen; Color T: True color; Chlo-a: Chlorophyll-a; Chlo-b: Chlorophyll-b; Chlo-c: Chlorophyll-c; Sal: Salinity; Sul: Sulfate; Turb: Turbidity; Color A: Apparent color; alka: Alkalinity; Nitrat: Nitrate.
Figure 4 - Biplot of the PCA showing relationships among physicochemical factors, sampling sites, and months
RELATIONSHIPS BETWEEN BIOLOGICAL AND ENVIRONMENTAL VARIABLES (RDA)
The RDA revealed clear spatiotemporal variation in cyanobacterial species as a function of environmental and climatic variables. The first two axes represented 47.9% of the variance (Figure 5). Significant variables included DO, temperature, EC, nitrate, and alkalinity. Axis 1 (34.1%) established temporal variation, with the March 2022 samples (positive quadrant) being associated with nitrate, alkalinity, and the coccoid species Aphanocapsa sp. and Aphanocapsa holsatica. In contrast, the September 2021 samples were associated with DO and filamentous species, such as Pseudanabaena galeata Böcher 1949, Planktothrix agardhii (Gomont 1892) Anagnostidis & Komárek 1988 emend. Gaget et al. 2015, and Planktolyngbya limnetica.
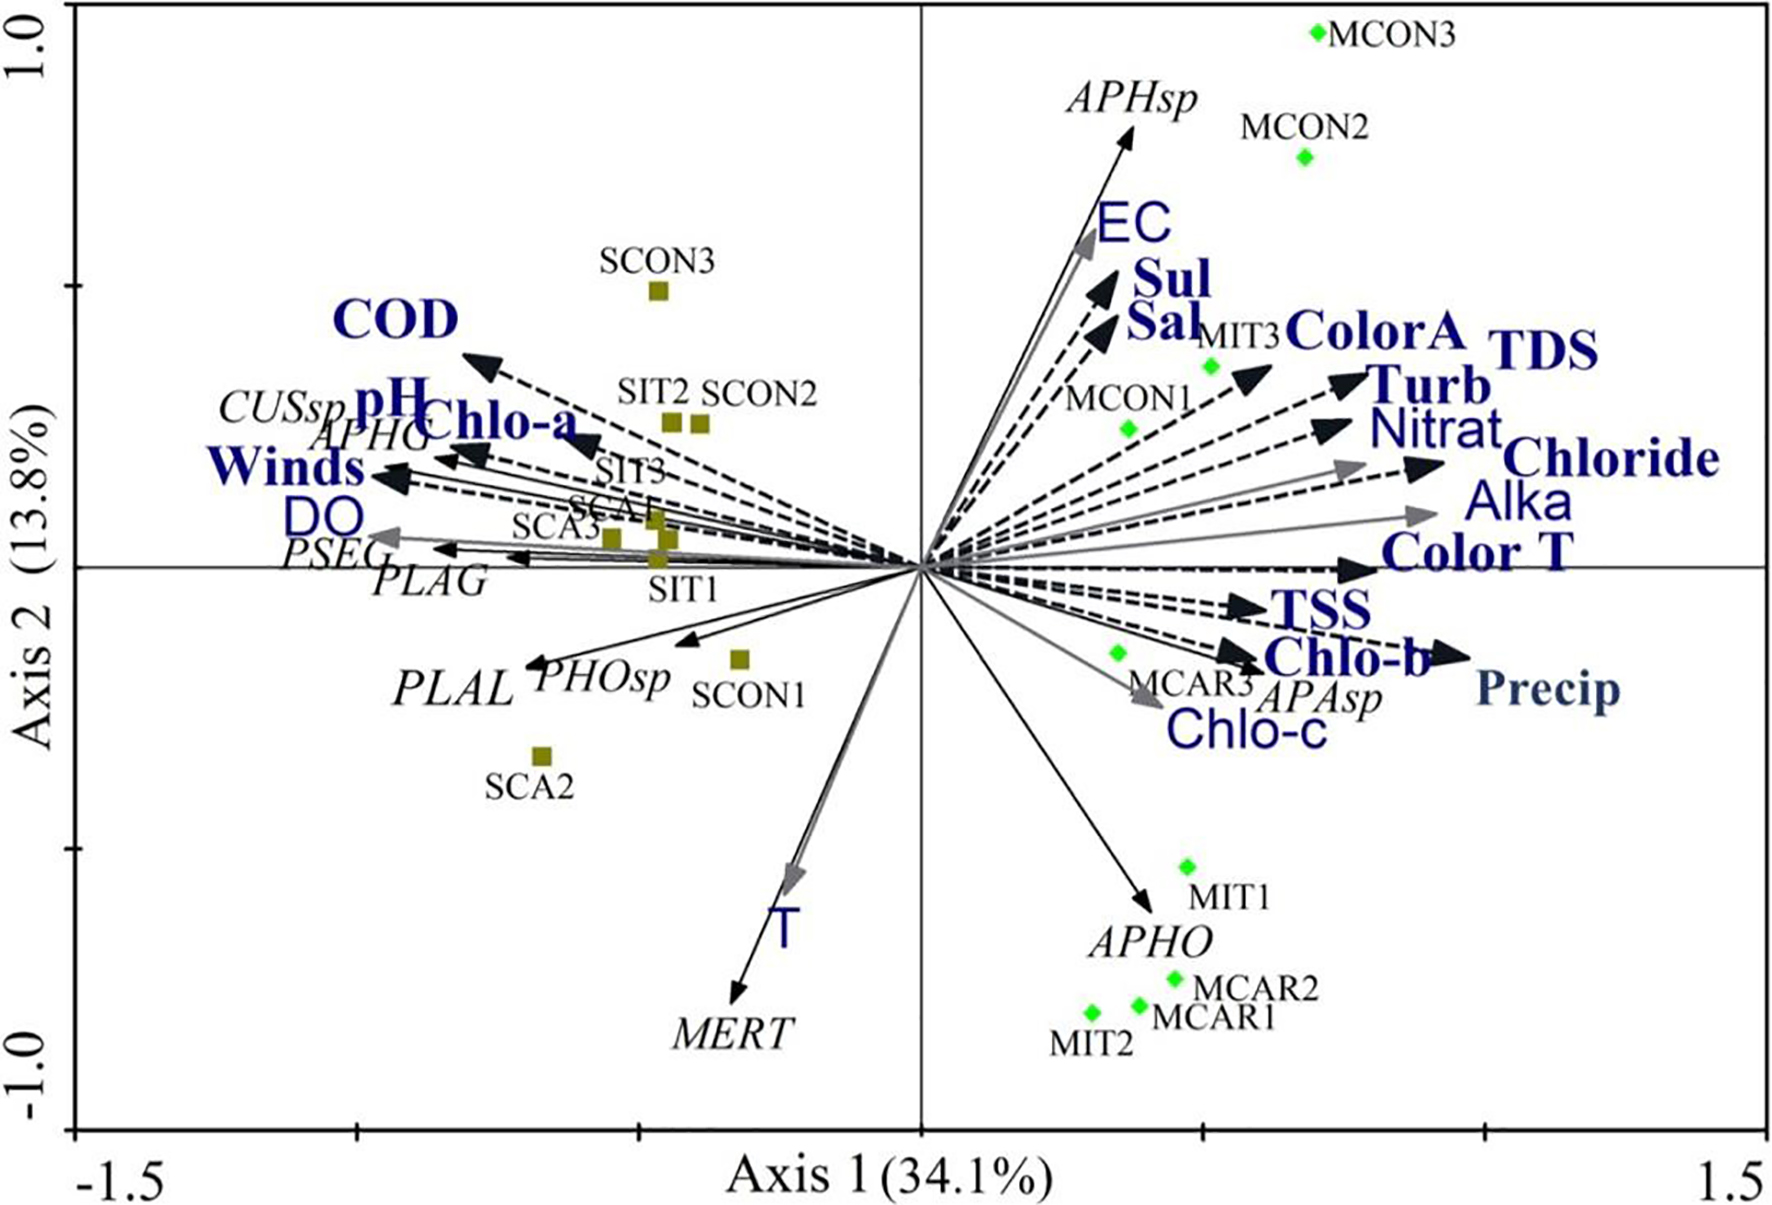
SCON: Conde Beach in September; SIT: Itupanema Beach in September; SCA: Caripi Beach in September; MCON: Conde Beach in March; MIT: Itupanema Beach in March; MCAR: Caripi Beach in March; PLAL: Planktolyngbya limnetica; PHOsp: Phormidium sp.; PLAG: Planktothrix agardhii; APHsp: Aphanizomenon sp. APHO: Aphanocapsa holsatica; MERT: Merismopedia tenuissima; CUSsp: Cuspidothrix sp.; PSEG: Pseudanabaena galeata; APAsp: Aphanocapsa sp.; APHG: Aphanizomenon gracile; COD: Chemical oxygen demand; TSS: Total suspended solids; Chlo-a: Chlorophyll-a; Chlo-b: Chlorophyll-b; Chlo-c: Chlorophyll-c; Color T: True color; Color A: Apparent color; EC: Electrical conductivity; Turb: Turbidity; DO: Dissolved oxygen; Nitrat: Nitrate; TDS: Total dissolved solids; Sal: Salinity; Sul: Sulfate; Alka: Alkalinity; Precip: Precipitation; pH: Hydrogen potential; T: Temperature.
Figure 5 - Triplot of physicochemical, climatic, and biological variables for Amazonian fluvial-estuarine beaches in Barcarena, Pará State, Brazil
Axis 2 (13.8%) differentiated Conde and Caripi beaches, with Itupanema Beach serving as a transition site between them. EC was the main variable influencing species distribution at Conde Beach, whereas temperature was more strongly associated with Caripi Beach.
DISCUSSION
In Pará, Amazon Region, studies on cyanobacteria are still scarce and were initially included only in phytoplankton community surveys, representing less than 10% of the composition, with many taxa described only at the genus level35,36. Since the first decade of the 21st century, research on this group has intensified, focusing mainly on species composition, density, blooms, cyanotoxin production, and their implications for human and environmental health13,19,37,38.
The species Anagnostidinema amphibium, Merismopedia tenuissima, and Planktolyngbya limnetica were frequent in both sampling periods and occurred on all beaches. Gomes et al.19 also reported Merismopedia tenuissima in Pará River, suggesting a good adaptation of this taxon to local conditions. The presence of a mucilaginous sheath enables its vertical positioning in the water column, a factor associated by Dunck et al.39 with its dominance in lacustrine environments.
On the other hand, Anagnostidinema amphibium [= Geitlerinema amphibium (Agardh ex Gomont 1892) Anagnostidis 1989] had not been frequently recorded in studies conducted in the Pará River estuary; yet, it was detected at all sampled beaches of the present study. This filamentous cyanobacterium, although non-bloom-forming, has been reported in Brazilian water supply sources40,41, exhibiting toxic potential demonstrated in experimental studies42. The species is also recorded in the cyanobacteria checklists for Pará State9,43.
Planktolyngbya limnetica showed the highest density recorded in September 2021 and was present on all beaches. In a study conducted in the Guarapiranga Reservoir (São Paulo State, Brazil), P. limnetica also showed higher density during the dry period, which was correlated with ammonium ion (NH₄⁺) concentrations in eutrophic environments44. In Pará State, this species has been recorded in freshwater systems⁹, and the present study thus documents its occurrence in low-salinity estuarine environments.
Filamentous species predominated in September, whereas coccoid forms were more common in March, consistent with a previous regional study15. The dominance of Planktolyngbya limnetica, a benthic freshwater species20, may be explained by local hydrodynamics, as wave movements towards the littoral region resuspend benthic forms from the sand surface to the water surface, an effect intensified in September, a period of strong winds.
Vila do Conde Beach is shaped like a cove and has numerous residences in its surroundings. It is also located near the port area, which is marked by intense transatlantic ship traffic and an industrial complex. In this area, there is a high density of other microalgae indicative of organic matter decomposition, although these organisms were not the focus of this study. Previous research at this site recorded the highest densities of Microcystis spp. and cyanotoxin production from January to April 202111,45. A limitation of the present study lies in not including other microalgal groups, which could provide a more comprehensive and assertive approach to the environmental and anthropogenic effects on this ecosystem.
Although this study covered the period from 2021 to 2022, recent temperature records in Barcarena, particularly in 2024, when more than 177 days of extreme heat were recorded and urban expansion reduced vegetation cover46, raise concerns about the intensification of cyanobacterial blooms under climate change scenarios. This trend suggests that the blooms observed between January and April 202111,45 may become more frequent and intense due to global warming and local hydrological changes. This aligns with the discussions of Zepernick et al.47, who highlight how rising temperatures, intensified thermal stratification, and extreme weather events promote the expansion and transport of toxic cyanobacterial blooms along the aquatic continuum, from rivers to estuaries and coastal environments.
Water quality in the Pará River, which borders the studied beaches, was found to be adequate for recreational activities during the study period according to CONAMA Resolutions No. 274 and 357 parameters, as no cyanobacterial blooms were detected.
Spatiotemporal variations in physicochemical parameters were observed through PCA and RDA analyses. Seasonal differences in these parameters were also reported by Piratoba et al.22 in the same area as the present study, identifying rainfall as a diluting factor for variables such as TDS, EC, and color, which showed lower concentrations during rainy months. In contrast, the present study recorded higher values of these parameters in March, suggesting that, in this context, rainfall intensifies the transport of organic matter and nutrients from the continent to water bodies. This additional input is associated with reduced DO levels (< 5 mg·L⁻¹) in March, confirming the rainy season as the most critical period for water quality.
Gomes et al.19 conducted a seasonal and interannual study (2009-2010) of the Pará River, finding that the seasonal effect can vary from year to year. In April 2009, rainfall acted as a diluting factor, and in July, the highest concentrations of nutrients, EC, TDS, and salinity were recorded for the area. In 2010, the opposite occurred: in April, the highest salinity and nutrient values were observed along with low DO levels, while August exhibited increased DO concentrations. This suggests that the Amazonian environment is dynamic and strongly influenced by the rainfall regime.
In the biotic and abiotic association (RDA), Aphanocapsa sp. and Aphanocapsa holsatica were associated with nitrate and alkalinity. Lawson et al.48 suggest that greater nutrient availability, including nitrogen, is positively related to the development of coccoid species such as Aphanocapsa. This genus is common in proliferations within tropical reservoirs, where longer hydrological retention times promote water column stability. In addition, the accumulation of nutrients in hypolimnetic zones may favor ecophysiological advantages for Aphanocapsa49. However, little is known about its dynamics in estuarine areas such as the Pará River, representing an important gap to be explored in future research in the region.
In the present study, Pseudanabaena galeata, Planktothrix agardhii, and Planktolyngbya limnetica were associated with the September samples, showing a correlation with DO values. This behavior may be attributed to the benthic habits of these species, favored by wave action in beach areas that enhances water and sandy sediment interaction. Strong winds recorded during this period likely further intensified water oxygenation, increasing DO availability in the water column. Similar findings were reported by Gomes et al.19, who also observed a higher representation of filamentous species during the dry season.
CONCLUSION
The present study expanded the knowledge on the diversity and dynamics of cyanobacteria on the beaches of Barcarena, identifying 41 species, 14 of which are potentially toxic. Clear seasonal patterns were observed, with higher cyanobacterial density during the dry season and greater species richness during the rainy season. These findings indicate a strong influence of physicochemical factors, such as dissolved oxygen, temperature, EC, nitrate, and alkalinity, on species distribution.
Although the beaches are currently classified as suitable for bathing, the presence of multiple potentially toxic species suggests possible risks to public and environmental health. Therefore, this study emphasizes the need for continuous monitoring and complementary research on toxicity, population dynamics, and environmental management strategies to support the safety of recreational activities, the conservation of aquatic ecosystems, and the advancement of regional scientific knowledge on cyanobacteria.

